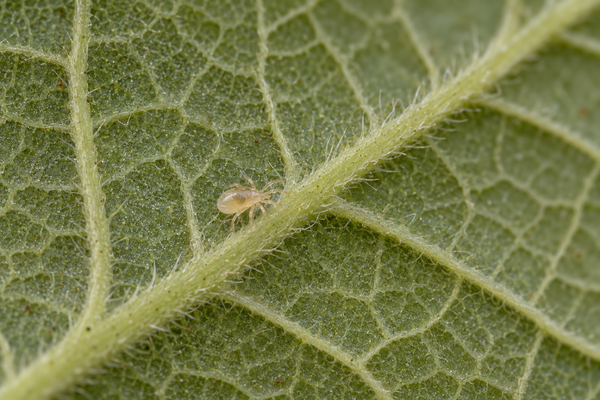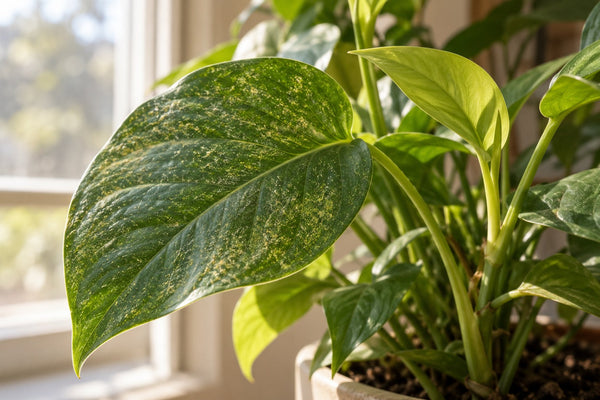


You can see whitefly when you walk past the plants. Under the leaves, there are eggs, settled young, and adults ready to leave. A predator that eats whitefly sounds like the answer—until you ask which of those stages it can eat.
That is the timing problem this article follows. Early releases let swirskii meet vulnerable young stages as they appear. Releasing into a dense established colony asks it to work around a much larger population, including stages it handles poorly.
Two greenhouse studies make the difference tangible: an early swirskii program on zucchini and a separate trial on dense whitefly colonies on cucumber. They are different experiments, not a matched early-versus-late test, but together they explain why the starting population matters.
The trial where the mite beat the sprayer
Almería, Spain, in a replicated experimental greenhouse. Three whole strategies against whitefly on zucchini: a biological program using nothing but swirskii, a conventional program of two sprays a week, and an integrated program of mites plus one biorational spray a week. The mites arrived in sachets (slow-release packets that hold a breeding colony) placed on the seedlings three days before transplant.
Whiteflies per leaf, week seven
Swirskii alone: 12.27. Integrated: 24.46. Conventional, two sprays a week: 41.97.
Read plainly
Mites placed on the plants three days before they went in the ground beat twice-weekly spraying on whitefly density, by a factor of about 3.4.
The mites were already on the seedlings before transplant. Keep that head start attached to the result when thinking about an established outbreak.
The one rescue test
Medd and GreatRex asked a commercial question. Can you treat a whitefly hot-spot with predatory mites? They used dense greenhouse whitefly (Trialeurodes vaporariorum) on cucumber, high mite inoculations, three species, loose product and sachets.
Plots treated with limonicus or montdorensis as loose product had significantly fewer whitefly throughout the trial. Swirskii is not listed among them. The authors were careful in their own conclusion, so it is worth keeping their shape. No species was clearly identified as a suitable candidate for treating high-density whitefly colonies, though the results suggest the highest level of predation in limonicus.
One finding from that paper is easy to skip. No species gathered on the leaves with the most whitefly. Released mites do not sniff out the outbreak and converge on it. They spread out and eat whatever they walk into.
So what do you do about a colony you can already see?
For whitefly that is already dense, the swirskii bottle is the wrong tool, and no rate makes it the right one. On the only same-protocol test, limonicus was the better mite, and the authors still declined to call any of the three suitable. The sequence every successful trial describes is to bring the standing population down some other way, then put swirskii into what is left so it does not rebuild.
Why more mites does not change the answer
A timing rule with no mechanism behind it is a superstition. This one has a mechanism, and it is measured.
Whitefly development runs from the egg through four nymphal instars to the winged adult. The fourth instar includes the stage growers call the pupa. Swirskii is most useful against the early part of that sequence.

| Whitefly stage | Can swirskii reach it? | The measurement |
|---|---|---|
| Egg | Yes | 30% of ten eggs eaten over five days by a single female, about 0.6 per mite per day (Cuthbertson 2014) |
| First instar, the crawler, the only nymph that walks | Yes | 27% over five days in the same test |
| Second instar | Barely | 8.5% in the same test, a significant drop. Second and later instars are about ten times less vulnerable than eggs and crawlers (Nomikou 2004) |
| Third instar | Not in practice | Not separately tested. The group that measured the collapse calls later instars invulnerable (Meng 2012) |
| Fourth instar, the "pupa" | Not in practice | Not separately tested. Larger and more thickened again |
| Adult | No | It flies. Stated in the papers that measured the immature stages rather than tested directly, but a winged insect is not prey for a wingless mite |
The drop comes between the first and second instar, the moment the nymph settles down and thickens. That rules out the easy explanation that the mite can only catch what moves. The crawler is the most mobile immature stage and gets eaten readily, and the settled second instar is the one that gets away. Size and cuticle fit the data. Wax and hardened shell get repeated everywhere as the cause, but nobody has measured them for this mite, so we will not state them as fact.
Now compare that with what an outbreak is made of. A whitefly population you can see across the room is mostly later nymphs on the undersides of older leaves, plus adults in the air. Those are exactly the stages the mite cannot get at. Adding mites raises the number of mites hunting the two stages it could already reach. It does not add a stage. A bottle buys speed of arrival, not a different diet.
Thrips follow the same shape, with six stages and one reachable, worked through attack by attack in the first-instar article.
The one thing the mite does to adults
Adult whiteflies that have watched a predator eat their offspring tend to leave plants that have predators on them. The effect is weak. Adults left predator plants faster when the neighboring plant was 0.6 m away but not when it was 2 m away, and the share that dispersed was low either way (Meng 2012).
A real behavior, and not a control method. Nothing in a swirskii release kills an adult whitefly.
A population, not an appetite
Picture one adult female mite in a small arena with a leaf disc, ten whitefly eggs and nothing else to eat. Five days pass. She has eaten three eggs.
That is about 0.6 whitefly eggs per mite per day, in conditions that flatter her: no plant to search and the prey stacked up in front of her. Swirskii was never an appetite. In the same study, swirskii, montdorensis and limonicus did not differ significantly on any single whitefly stage, so it is not a standout at eating whitefly eggs either.
What it does have is a numerical response, which means its population grows when food is around. It feeds and breeds on pollen, so it can hold a standing population on a plant that has no pest on it at all. That is the only reason a preventive release is possible. A specialist predator starves between outbreaks, and this one does not. Someone even tested whether feeding it pollen would dilute its control of whitefly, and adding pollen improved control through the whole experiment (Nomikou 2010).
So what a preventive program buys is a population that arrives early and stays. Bought as a response to something you can already see, it is 0.6 eggs a day against a colony made mostly of stages it cannot eat.
A density drop is not a virus drop
Go back to the zucchini trial. Swirskii alone gave the lowest whitefly density of the three strategies, 12.27 per leaf against 41.97 for spraying. The same trial also measured tomato leaf curl New Delhi virus, which whitefly carries. On virus suppression the order flipped: integrated 73%, biological 58%, conventional 44%.
The strategy with the fewest whiteflies was not the strategy with the least virus. A virus can move at whitefly densities far below anything control reaches, because it takes very few insects to infect a plant.

Someone buying swirskii to stop a virus is buying the wrong thing. Density control and disease control come apart at exactly the densities that matter for disease.
It has shown up by a second route
A tomato study bred lines that make acylsugars, sticky compounds that suppress whitefly on their own. Those lines carried fewer whiteflies, and yet tomato yellow leaf curl virus was detected more often in them than in the commercial lines in the field (Pandey 2023).
Two interventions, two crops, two viruses, and the same split. The insect count fell and the disease did not follow, which points to virus transmission rather than to anything about predatory mites.
If your problem is whitefly feeding, honeydew and sooty mold, a preventive swirskii program beat a conventional spray program in a replicated trial. If your problem is a virus in a crop where one infected plant is a write-off, the mite is one component behind exclusion (screening, clean starts, keeping the vector out of the house), and more mites is not the lever.
What this says about thrips
Most people reading this bought swirskii for thrips, so the edge of the argument matters. The mechanism carries across. Under direct observation of individual attacks, swirskii failed against every second-instar larva of three thrips species and took the first instar (Beretta 2024). So on thrips too it works on the generation coming up behind the one you can see, and the count falls over a couple of weeks rather than overnight.
The trial record does not carry across, and here it is friendlier. A single release of 30 mites per plant held chilli thrips below one per terminal leaf for 28 days, against up to 36 for cucumeris and 70 for untreated plants in the same experiment (Arthurs 2009). Nobody has run the Medd and GreatRex design on thrips, so the rescue result belongs to whitefly and we will not lend it to a pest it was not measured on. For active thrips, a bottle is the format built for it.
References
- Cuthbertson, A.G.S. (2014). The feeding rate of predatory mites on life stages of Bemisia tabaci Mediterranean species. Insects 5: 609–614. doi.org
- Nomikou, M., Janssen, A., Schraag, R. & Sabelis, M.W. (2004). Vulnerability of Bemisia tabaci immatures to phytoseiid predators: consequences for oviposition and influence of alternative food. Entomologia Experimentalis et Applicata 110: 95–102. doi.org
- Nomikou, M., Janssen, A., Schraag, R. & Sabelis, M.W. (2002). Phytoseiid predators suppress populations of Bemisia tabaci on cucumber plants with alternative food. Experimental and Applied Acarology 27: 57–68. doi.org
- Nomikou, M., Sabelis, M.W. & Janssen, A. (2010). Pollen subsidies promote whitefly control through the numerical response of predatory mites. BioControl 55: 253–260. doi.org
- Medd, N.C. & GreatRex, R.M. (2014). An evaluation of three predatory mite species for the control of greenhouse whitefly (Trialeurodes vaporariorum). Pest Management Science 70: 1492–1496. doi.org
- Rodríguez, E., Téllez, M.M. & Janssen, D. (2019). Whitefly control strategies against tomato leaf curl New Delhi virus in greenhouse zucchini. International Journal of Environmental Research and Public Health 16: 2673. doi.org
- Calvo, F.J., Bolckmans, K. & Belda, J.E. (2011). Control of Bemisia tabaci and Frankliniella occidentalis in cucumber by Amblyseius swirskii. BioControl 56: 185–192. doi.org
- Calvo, F.J., Bolckmans, K. & Belda, J.E. (2009). Development of a biological control-based Integrated Pest Management method for Bemisia tabaci for protected sweet pepper crops. Entomologia Experimentalis et Applicata 133: 9–18. doi.org
- Abou Jawdah, Y., Ezzeddine, N., Fardoun, A., Kharroubi, S., Sobh, H., Atamian, H.S., Skinner, M. & Parker, B. (2024). Biological control of three major cucumber and pepper pests in high plastic tunnels using two local phytoseiid mites. Plants 13: 889. doi.org
- Meng, R.-X., Sabelis, M.W. & Janssen, A. (2012). Limited predator-induced dispersal in whiteflies. PLoS ONE 7: e45487. doi.org
- Beretta, G.M., Zandbergen, L., Deere, J.A., Messelink, G.J., Muñoz Cárdenas, K. & Janssen, A. (2024). Predator–prey interactions: how thrips avoid predation. Biological Control 188: 105437. doi.org
- Arthurs, S., McKenzie, C.L., Chen, J., Doğramacı, M., Brennan, M., Houben, K. & Osborne, L. (2009). Evaluation of Neoseiulus cucumeris and Amblyseius swirskii as biological control agents of chilli thrips on pepper. Biological Control 49: 91–96. doi.org
- Paspati, A., Rambla, J.L., López Gresa, M.P., Arbona, V., Gómez-Cadenas, A., Granell, A., González-Cabrera, J. & Urbaneja, A. (2021). Tomato trichomes are deadly hurdles limiting the establishment of Amblyseius swirskii. Biological Control 157: 104572. doi.org
- Pandey, S., da Silva, A.L.B.R., Dutta, B., Chong, J.H., Mutschler, M.A. & Schmidt, J.M. (2023). Acylsugar tomato lines suppress whiteflies and Amblyseius swirskii establishment. Entomologia Experimentalis et Applicata 171: 745–753. doi.org